
BIOL-321 · Lesson 6 of 12 · 28 min
Sexual selection and social evolution
Some of the most striking features of animals seem to make no sense for survival: the peacock’s enormous tail, the antlers of red deer, the songs of birds, the elaborate displays of manakins. Darwin recognized that these traits evolve because they help individuals win mates, a process he called sexual selection. Equally puzzling are behaviours that benefit others at a cost to oneself, such as the sterile workers of ant colonies or the alarm calls of ground squirrels. This lesson explains both through the logic of genes and fitness: sexual selection through competition and choice, and social behaviour through kin selection and evolutionary game theory.
Why the sexes differ
Sexual selection begins with anisogamy, the difference in size between gametes. Females, by definition, produce larger gametes (eggs) and males smaller ones (sperm). Because eggs are costly and sperm cheap, and because in many species females also invest more in parental care, female reproductive success is often limited by resources, while male success is limited by the number of mates. Angus Bateman studied fruit flies in 1948 and reported that male reproductive success increased steeply with the number of mates, while female success increased only slightly. The slope of reproductive success on mating success is now called the Bateman gradient.
import numpy as np
rng = np.random.default_rng(321)
# Simulated mating system: females gain a little from extra mates, males gain a lot (illustrative)
n = 500
f_mates = rng.poisson(1.5, n)
m_mates = rng.poisson(1.5, n) * rng.binomial(1, 0.7, n) + rng.poisson(0.3, n)
f_off = rng.poisson(8 + 1.0*np.minimum(f_mates, 2))          # females limited by egg production
m_off = rng.poisson(0.5 + 5.5*m_mates)                        # males limited by number of mates
for sex, x, y in [("females", f_mates, f_off), ("males", m_mates, m_off)]:
    rs = y / y.mean(); ms = x / x.mean()
    grad = np.polyfit(ms, rs, 1)[0]
print(f"{sex:7s}: variance in relative reproductive success = {rs.var():.2f}, Bateman gradient = {grad:.2f}")females: variance in relative reproductive success = 0.11, Bateman gradient = 0.11 males : variance in relative reproductive success = 1.10, Bateman gradient = 0.97
In this simulated system, males vary much more in reproductive success than females, and their Bateman gradient is steeper. The greater the variance in mating success, the stronger sexual selection can be. Later work found that Bateman’s original analysis had statistical problems, and that females in many species also gain from multiple mates, for example through genetic benefits or insurance against infertile partners. The general principle remains useful, but sex roles vary: in pipefish and seahorses, males brood the eggs, females compete for mates and females are more ornamented. What matters is which sex is more limited by access to mates, not which sex it is.
Competition and choice
Sexual selection works in two main ways. In intrasexual selection, members of one sex, usually males, compete directly for access to mates, favouring weapons such as antlers and horns, large body size and fighting ability. In intersexual selection, or mate choice, members of one sex, usually females, choose among potential partners, favouring ornaments and displays. Competition continues after mating: sperm competition favours large testes and rapid sperm in species where females mate with several males, and females may bias fertilization toward particular males, called cryptic female choice.
Why should females choose? Several explanations are not mutually exclusive. Females may gain direct benefits, such as food, territory or parental care. They may gain indirect, genetic benefits: either attractive sons (Fisher’s runaway process) or offspring with better overall genetic quality (good genes). And preferences may arise from sensory bias, a pre-existing preference in the female’s nervous system that males evolve to exploit. In water mites and some fish, females respond to stimuli resembling prey, and male displays imitate those stimuli.
Fisher’s runaway
Ronald Fisher argued in 1930 that once a female preference for a male trait becomes common, the trait and the preference can reinforce each other. Females that prefer long-tailed males have sons with long tails, which are attractive, and daughters who inherit the preference. Because the genes for the trait and the preference come to be associated in the offspring of choosy females (a genetic correlation), selection on the trait drags the preference along with it, and the process can run away until natural selection against extreme ornaments, through predation or energy costs, balances it.
import numpy as np
# A simple deterministic sketch of Fisherian runaway (after Lande 1981, highly simplified)
# t = mean male trait, p = mean female preference (both in SD units)
# Natural selection pulls t toward 0; sexual selection pushes t toward p.
# Genetic covariance B between t and p makes p change whenever t changes.
def run(B, gens=200, c=0.05, a=0.10, Gt=1.0):
    t, p = 0.1, 0.1
    for _ in range(gens):
        beta_t = a*p - c*t          # selection gradient on trait: attraction minus survival cost
        dt = Gt*beta_t
        dp = B*beta_t               # preference changes only by correlated response
        t, p = t + dt, p + dp
    return t, p

for B in (0.2, 0.4, 0.7):
    t, p = run(B)
print(f"genetic covariance {B}: after 200 generations trait = {t:8.2f}, preference = {p:8.2f}")genetic covariance 0.2: after 200 generations trait = 0.27, preference = 0.13 genetic covariance 0.4: after 200 generations trait = 0.53, preference = 0.27 genetic covariance 0.7: after 200 generations trait = 12.97, preference = 9.11
In this sketch, when the genetic covariance between trait and preference is small, the population soon stops changing: trait and preference settle at a point where the attraction of the trait to females exactly balances its survival cost. Lande showed that there is a whole line of such equilibria, so where a population ends up depends on where it started. Above a threshold covariance (0.5 with these settings), sexual selection outruns natural selection, and trait and preference escalate together. Russell Lande’s 1981 model showed that runaway can produce elaborate traits from arbitrary starting preferences, which may explain why closely related species can differ so dramatically in ornaments: the direction of runaway depends partly on chance.
Honest signals and the handicap principle
If ornaments only advertised attractiveness, males might cheat by producing cheap displays. Amotz Zahavi proposed in 1975 that ornaments are reliable because they are costly: only high-quality males can afford a large tail or an exhausting display, so the ornament is an honest signal of quality. The handicap principle was controversial at first, but Alan Grafen showed mathematically in 1990 that costly signals can be evolutionarily stable when the cost is higher for low-quality individuals. Evidence includes the carotenoid-based red colouring of male house finches and three-spined sticklebacks: carotenoids must be obtained from food and are also needed for immune function, so bright colour indicates good foraging and health. Female house finches prefer redder males, which tend to be better fathers.
| Mechanism | What the chooser gains | Example |
|---|---|---|
| Direct benefits | Resources, protection, parental care | Nuptial gifts in crickets and scorpionflies |
| Fisherian runaway | Attractive sons | Long tails of widowbirds (Andersson 1982 tail-lengthening experiment) |
| Good genes / handicap | Offspring of higher genetic quality | Carotenoid colour in house finches and sticklebacks |
| Sensory bias | None; preference predates the trait | Swordtail fish: females of related swordless species prefer males with artificial swords |
Malte Andersson’s 1982 experiment on long-tailed widowbirds in Kenya is a classic test. He cut the tails of some males and glued the pieces onto others, extending them by about 25 cm. Males with lengthened tails attracted more nesting females than control males or males with shortened tails, showing that females prefer longer tails than those that currently exist.
Kin selection and Hamilton’s rule
Natural selection favours genes that increase their own transmission. W. D. Hamilton realized in 1964 that a gene can do this not only by helping the individual carrying it reproduce, but also by helping relatives, who carry copies of the same gene. An altruistic act, one that costs the actor C in offspring but gives a recipient B extra offspring, will be favoured if rB > C, where r is the coefficient of relatedness, the probability that a gene in the actor is also present in the recipient by recent common descent. The total effect of a gene on copies of itself in the actor and in relatives is called inclusive fitness. J. B. S. Haldane reportedly anticipated the idea with the joke that he would lay down his life for two brothers or eight cousins.
Worked problem
Should a ground squirrel give an alarm call?
A female Belding’s ground squirrel sees a predator. Calling raises her own risk of being caught, costing on average 0.1 future offspring. If she calls, her three nearby daughters and her two nieces each gain 0.04 future offspring from escaping. Is calling favoured by kin selection?
Show solution
- Relatedness: daughter r = 0.5; niece r = 0.25.
- Benefit weighted by relatedness: 3 × 0.5 × 0.04 + 2 × 0.25 × 0.04 = 0.06 + 0.02 = 0.08.
- Cost to self = 0.1.
- Since 0.08 < 0.1, Hamilton’s rule is not satisfied in this case; if she had more close kin nearby, calling would be favoured.
Answer: Not in this example (rB = 0.08 < C = 0.10); field studies by Paul Sherman found that females with close kin nearby call more often, as the rule predicts.
Kin selection explains much social behaviour. Helpers at the nest, common in cooperatively breeding birds such as Florida scrub-jays, are usually offspring from previous years helping their parents raise siblings. Many animals can recognize kin, by familiarity or by cues such as odour, and direct help toward them. In the social insects, sterile workers raise their mothers’ offspring. Hamilton noted that in Hymenoptera (ants, bees and wasps), males are haploid, so full sisters share three-quarters of their genes, more than mothers and daughters share. This haplodiploidy hypothesis was once thought to explain why eusociality evolved so often in Hymenoptera, but it is now considered insufficient on its own: termites, which are diploid, are also eusocial, and many queens mate with several males, lowering relatedness among workers. Ecological factors, such as defensible nests and the benefits of group living, and a history of monogamy in ancestors, appear to be important too.
Evolutionary game theory
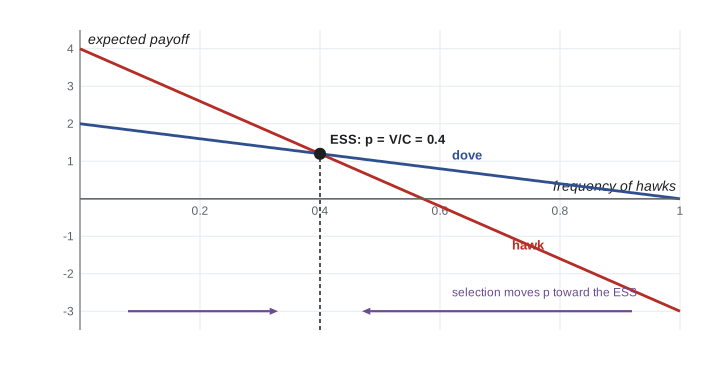
When the best strategy depends on what others do, evolution can be analysed as a game. John Maynard Smith and George Price introduced the evolutionarily stable strategy (ESS) in 1973: a strategy that, once common, cannot be invaded by any rare alternative. The classic example is the hawk–dove game. Two individuals contest a resource of value V. Hawks always escalate; doves display and retreat if attacked. Two hawks fight, and the loser pays a cost C; two doves share the resource; a hawk always beats a dove.
import numpy as np
# Hawk–dove payoffs to the row player
V, C = 4.0, 10.0
payoff = np.array([[(V - C)/2, V],      # hawk vs hawk, hawk vs dove
                   [0.0,       V/2]])   # dove vs hawk, dove vs dove
# Replicator dynamics for the frequency of hawks, p
p = 0.9
for t in range(300):
    f_h = p*payoff[0, 0] + (1 - p)*payoff[0, 1]
    f_d = p*payoff[1, 0] + (1 - p)*payoff[1, 1]
    fbar = p*f_h + (1 - p)*f_d
    p = p + 0.05*p*(f_h - fbar)
print(f"V = {V}, C = {C}: replicator dynamics converge to hawk frequency {p:.3f}; ESS theory predicts V/C = {V/C:.3f}")
for C2 in (2.0, 4.0, 20.0):
print(f"cost {C2:4.1f}: ESS hawk frequency = {min(1.0, V/C2):.2f}")V = 4.0, C = 10.0: replicator dynamics converge to hawk frequency 0.400; ESS theory predicts V/C = 0.400 cost 2.0: ESS hawk frequency = 1.00 cost 4.0: ESS hawk frequency = 1.00 cost 20.0: ESS hawk frequency = 0.20
If the cost of fighting exceeds the value of the resource, neither pure strategy is stable: a population of doves is invaded by hawks, which win every contest, but a population of hawks is invaded by doves, which avoid costly fights. The ESS is a mixture with hawks at frequency V/C. When fighting is cheap relative to the prize, always being a hawk is the ESS. Game theory explains why most animal contests are settled by display rather than injury, why strategies such as conditional and alternative mating tactics persist and how cooperation can evolve between unrelated individuals through reciprocity, when the same individuals interact repeatedly, as Robert Axelrod’s tournaments of the repeated prisoner’s dilemma showed.
Conflict within families and genomes
Kin selection also predicts conflict. Because parents are equally related to all their offspring but each offspring is more related to itself than to its siblings, offspring are expected to demand more care than parents are selected to give, a parent–offspring conflict described by Robert Trivers in 1974. This idea helps explain weaning conflicts and even the battle over nutrients between mother and fetus in mammals. Genomic imprinting (BIOL-201) may reflect a similar conflict: genes inherited from the father, which benefit from extracting more maternal resources, such as the growth factor IGF2, are expressed, while maternally inherited copies are silenced, and vice versa for genes that limit growth, as David Haig proposed. Conflicts can occur even within a genome, when selfish genetic elements, such as transposable elements and meiotic drivers, spread at the expense of the organism carrying them.
Common mistakes
MistakeSexual selection always means females choose and males compete.
InsteadRoles depend on which sex is limited by mates; in pipefish and seahorses, females compete and males choose.
MistakeOrnaments exist because they help survival.
InsteadOrnaments often reduce survival but increase mating success.
MistakeAn altruistic behaviour cannot evolve by natural selection.
InsteadIt can, if rB > C, through kin selection, or through reciprocity among repeated partners.
MistakeRelatedness r is the fraction of all genes two relatives share.
Insteadr is the probability that a gene is shared by recent common descent, beyond the background similarity of the population.
MistakeHaplodiploidy fully explains eusociality.
InsteadDiploid termites are eusocial and multiple mating lowers worker relatedness; ecology and monogamy also matter.
MistakeAn evolutionarily stable strategy maximizes the average fitness of the population.
InsteadAn ESS cannot be invaded by rare alternatives; it need not maximize population fitness.
Summary and key terms
- Anisogamy and unequal parental investment usually make one sex more limited by mates, creating higher variance in mating success and stronger sexual selection.
- Intrasexual competition favours weapons and size; intersexual choice favours ornaments and displays; competition continues after mating.
- Mate choice can be explained by direct benefits, Fisherian runaway, honest handicap signals or sensory bias.
- Hamilton’s rule rB > C shows that altruism is favoured when benefits to relatives, weighted by relatedness, exceed the cost to the actor.
- Kin selection explains alarm calls, helpers at the nest and worker sterility, though eusociality also depends on ecology and monogamy.
- An ESS cannot be invaded by rare strategies; in the hawk–dove game, hawks persist at frequency V/C when fights are costly.
- Kin selection also predicts conflict, between parents and offspring and between maternally and paternally inherited genes.
- sexual selection
- Selection arising from differences in mating success.
- anisogamy
- The difference in size between male and female gametes.
- Bateman gradient
- The slope of reproductive success on mating success.
- intrasexual selection
- Competition within one sex for access to mates.
- mate choice
- Preference by members of one sex for particular partners.
- Fisherian runaway
- Coevolution of a trait and a preference reinforcing each other through genetic correlation.
- handicap principle
- The idea that costly signals are honest indicators of quality.
- inclusive fitness
- An individual’s own reproduction plus its effects on relatives’ reproduction weighted by relatedness.
- Hamilton’s rule
- Altruism is favoured when rB > C.
- evolutionarily stable strategy
- A strategy that, when common, cannot be invaded by a rare alternative.
Practice problems
Work each problem on paper first, then reveal the answer to check.
Why are males often the more ornamented sex?
Show answer
Males are usually more limited by access to mates, so variance in their mating success and sexual selection are stronger.
What is sperm competition, and what trait does it favour?
Show answer
Competition among sperm from different males to fertilize eggs; it favours large testes and many or fast sperm.
What did Andersson’s widowbird experiment show?
Show answer
Males with artificially lengthened tails attracted more females, so females prefer longer tails.
Why can a costly ornament be an honest signal?
Show answer
Only high-quality individuals can afford the cost, so cheating does not pay.
Calculate rB for helping two full siblings each gain 0.3 offspring.
Show answer
rB = 0.5 × 0.6 = 0.3.
In haplodiploid Hymenoptera, what is the relatedness between full sisters?
Show answer
0.75.
In the hawk–dove game with V = 6 and C = 12, what is the ESS frequency of hawks?
Show answer
V/C = 0.5.
When is always playing hawk an ESS?
Show answer
When the value of the resource is at least as large as the cost of fighting (V ≥ C).
What is parent–offspring conflict?
Show answer
Disagreement over parental investment because offspring value themselves more than siblings, while parents value all offspring equally.
How might imprinting reflect genetic conflict?
Show answer
Paternally inherited genes favour extracting more maternal resources, so growth-promoting genes such as IGF2 are expressed from the paternal copy.
Lesson quiz · 5 questions
Score 60% or more to complete this lesson.
Create a free account to save your progress, take quizzes and earn a certificate.