
BIOL-350 · Lesson 11 of 12 · 32 min
Osmoregulation and excretion
Life began in the sea, and the cells of every animal still work in a salty fluid. Animals that moved into fresh water and onto land took the problem of keeping that fluid right with them. A freshwater fish is saltier than its surroundings and constantly gains water and loses salt; a marine fish is more dilute than sea water and constantly loses water and gains salt; a land animal loses water to dry air with every breath. All of them must also get rid of the nitrogen released when they break down proteins, and nitrogenous wastes have their own costs. This lesson explains osmoregulation, the control of the water and salt content of body fluids, and excretion, the removal of metabolic wastes, from marine invertebrates to the mammalian kidney. Lesson 1 introduced osmoconformers and osmoregulators; here we look at how regulation works.
Osmosis, osmolarity and tonicity
Water moves across a semipermeable membrane from a solution of lower total solute concentration to one of higher concentration, a process called osmosis. The total concentration of osmotically active particles is the osmolarity (per liter of solution) or osmolality (per kilogram of water), measured in osmoles. One mole of glucose gives about one osmole, one mole of sodium chloride about two, because it dissociates into two ions (slightly less in practice, because of ion interactions). Sea water has an osmolality of about 1,000 mOsm per kg; fresh water is usually below 10; mammalian plasma about 290 to 300; and marine teleost fish about 350 to 400. The osmotic pressure of a solution, the pressure needed to stop water from flowing into it from pure water, is given approximately by the van 't Hoff equation.
Osmolarity is a property of a solution; tonicity describes what a solution does to a cell placed in it. A solution is hypotonic to a cell if the cell swells in it, hypertonic if the cell shrinks, and isotonic if its volume does not change. Tonicity depends on which solutes can cross the membrane: urea, which crosses membranes readily, adds to osmolarity but has little lasting effect on cell volume. Cells regulate their own volume by moving ions such as potassium and chloride and organic osmolytes such as taurine, betaine and sorbitol across their membranes.
Osmoconformers and the counteracting solutes of sharks
Most marine invertebrates, such as sea stars, mussels and squid, are osmoconformers: their body fluids are close to sea water in osmolality, though they regulate the concentrations of particular ions, keeping sulfate and magnesium low, for example. Their cells match the osmolality of the body fluid largely with organic osmolytes such as free amino acids, which do not disturb protein function the way high concentrations of salts would.
Sharks, skates, rays and the coelacanth use a different solution. Their plasma has a salt concentration only about a third that of sea water, but they retain high concentrations of urea, about 350 to 400 mM, which brings their total osmolality slightly above that of sea water. As a result, they gain a little water by osmosis rather than losing it, and the excess is excreted by the kidney. Urea at such concentrations would destabilize proteins, but elasmobranchs also accumulate trimethylamine oxide (TMAO), a methylamine that counteracts the effect of urea on proteins, in a ratio of about two urea to one TMAO. Excess salt is excreted by a rectal gland. This counteracting-solute strategy was described by Paul Yancey and George Somero in 1979. TMAO also increases with depth in deep-sea fish, where it appears to counteract the destabilizing effect of high hydrostatic pressure on proteins.
Fish in fresh water and sea water
Bony fish keep their plasma at about a third of the osmolality of sea water in both fresh and salt water, so they face opposite problems in the two environments. A freshwater fish gains water by osmosis across its gills and loses ions by diffusion. It excretes the excess water as copious dilute urine, up to a third of its body mass per day in some species, and actively takes up sodium and chloride across the gills through specialized ionocytes, also called mitochondria-rich cells or chloride cells, and from food. A marine teleost loses water to the sea and gains salt. It drinks sea water, absorbs water across the gut by first absorbing salt, excretes divalent ions such as magnesium and sulfate in small volumes of urine, and actively secretes the excess sodium and chloride across the gills through ionocytes of a different type, powered by the sodium pump.
Euryhaline fish can move between fresh and salt water. Atlantic salmon hatch in rivers in Quebec, the Maritimes, Newfoundland and Maine, spend one to three years in fresh water, and then undergo smoltification, a set of changes that prepare them for the sea. Under the control of photoperiod, cortisol, growth hormone and thyroid hormones, young salmon change color to silver, increase the number of seawater-type ionocytes and the expression of sodium pumps in their gills, and begin to drink. On their return to spawn, the hormone prolactin promotes the freshwater pattern again. Pacific salmon, the American eel, which spawns in the Sargasso Sea and grows in rivers along the Atlantic coast, and the stickleback offer further examples. Stickleback populations have repeatedly colonized fresh water from the sea since the last glaciation, and the same genes have been involved repeatedly, a case study in parallel evolution.
# Osmotic water gain by a freshwater fish (teaching estimate)
R, T = 8.314, 283.15            # J per mol per K, 10 degC
plasma, water = 300.0, 5.0      # mOsm per kg
dpi = (plasma - water) * R * T  # osmotic pressure difference, Pa (mOsm/kg ~ mol/m^3)
print(f"osmotic pressure difference = {dpi/1e6:.2f} MPa = {dpi/101325:.1f} atm")

# Water influx through the gills, J = Lp * A * dpi
Lp = 2.0e-14          # hydraulic permeability of gill epithelium, m per s per Pa (illustrative)
A_per_kg = 0.25       # gill area, m^2 per kg body mass (typical active teleost)
mass = 0.5            # kg trout
J = Lp * A_per_kg * mass * dpi                    # m^3 per s
per_day_ml = J * 1e6 * 86400
print(f"water influx = {per_day_ml:.0f} mL per day = {100 * per_day_ml / (mass * 1000):.0f} % of body mass")
# the same flux must leave as urine; salt lost in urine at 10 mM NaCl
na_loss = per_day_ml / 1000 * 10.0
print(f"NaCl lost in urine at 10 mM: {na_loss:.1f} mmol per day, replaced by active uptake")osmotic pressure difference = 0.69 MPa = 6.9 atm water influx = 150 mL per day = 30 % of body mass NaCl lost in urine at 10 mM: 1.5 mmol per day, replaced by active uptake
Even with a fairly low hydraulic permeability, the osmotic gradient of about 0.7 MPa, roughly seven atmospheres, drives a large daily influx of water, which the kidney must excrete. Every milliliter of urine carries some salt, which must be replaced by active uptake at the gills. Freshwater fish reduce their losses by making very dilute urine, reabsorbing most of the filtered sodium and chloride in the kidney tubules, and by having gills with low permeability to water and ions compared with those of marine fish.
Nitrogenous wastes
When amino acids and nucleic acids are broken down, their nitrogen is released as ammonia, which is highly toxic: it disrupts pH and ion balance and interferes with neurotransmission in the brain. Animals excrete nitrogen in three main forms, and which they use depends largely on water availability. Ammonia is very soluble and diffuses readily across membranes, so most aquatic animals, including bony fish and aquatic invertebrates, excrete it directly into the water, mainly across the gills. Excreting ammonia needs large volumes of water to keep it dilute, about 400 mL per gram of nitrogen.
Urea, made from ammonia and carbon dioxide in the liver by the ornithine–urea cycle, discovered by Hans Krebs and Kurt Henseleit in 1932, is about 100,000 times less toxic, so it can be concentrated in body fluids and urine. Mammals, adult amphibians, sharks and some turtles excrete urea. Making it costs energy, about four ATP equivalents per molecule, but it saves water, needing about 50 mL per gram of nitrogen. Uric acid and its salts, excreted by birds, most reptiles and insects, are poorly soluble and precipitate as a paste, so they can be excreted with very little water, about 10 mL per gram of nitrogen, although synthesis is costlier. Uric acid excretion also suits development inside a shelled egg, where wastes must be stored in a closed space without poisoning the embryo: the precipitated uric acid stays out of solution in the allantois.
| Waste | Toxicity | Solubility | Water needed per g N (approx.) | Energy cost | Typical animals |
|---|---|---|---|---|---|
| Ammonia | High | Very high | 300–500 mL | Lowest | Bony fish, aquatic invertebrates, tadpoles |
| Urea | Low | High | about 50 mL | Moderate (urea cycle) | Mammals, adult amphibians, sharks |
| Uric acid | Very low | Very low (precipitates) | about 10 mL | Highest | Birds, most reptiles, insects, land snails |
The developmental switch in frogs illustrates the link with habitat. Tadpoles excrete ammonia into the pond; at metamorphosis, under the influence of thyroid hormone (lesson 7), the liver increases its urea cycle enzymes and the froglet switches to excreting urea. Lungfish, which survive droughts by burrowing into mud and forming a cocoon, switch from ammonia to urea when the water disappears, and some semi-terrestrial crabs and fish can do the same.
How kidneys work: filtration, reabsorption and secretion
Most animal excretory organs work in the same basic way. First, a filtrate of body fluid is formed, either by pressure filtration, as in the vertebrate glomerulus, or by secretion, as in insect Malpighian tubules. Then, as the fluid passes along a tubule, useful substances such as glucose, amino acids, most of the salt and water are selectively reabsorbed, and unwanted substances are secreted into it. Filtration followed by reabsorption may seem wasteful, but it has a great advantage: anything not specifically reabsorbed is excreted, so the kidney can clear novel toxins without needing a specific transporter for each one.
Insects use Malpighian tubules, blind-ended tubes that open into the gut. Their cells actively secrete potassium, and water and other solutes follow, forming a primary urine that passes into the hindgut, where the rectum reabsorbs most of the water and ions. Desert beetles and mealworms can reabsorb water from their feces so efficiently, using a cryptonephridial arrangement in which the Malpighian tubules are pressed against the rectum, that some can even absorb water vapor from humid air.
The mammalian nephron
The human kidney contains about a million nephrons. Each begins with a glomerulus, a tuft of capillaries inside a cup called Bowman's capsule, where blood pressure forces a protein-free filtrate out of the blood, driven by the Starling forces described in lesson 8. The two human kidneys filter about 180 liters of plasma per day, yet produce only 1 to 2 liters of urine, so more than 99 percent of the filtered water is reabsorbed. The proximal tubule reabsorbs about two thirds of the filtered salt and water, all of the glucose and amino acids, and most of the bicarbonate, by active transport of sodium followed by water. Next comes the loop of Henle, which dips from the cortex into the medulla and back. Then the distal tubule and collecting duct fine-tune the composition of the urine under hormonal control.
The countercurrent multiplier
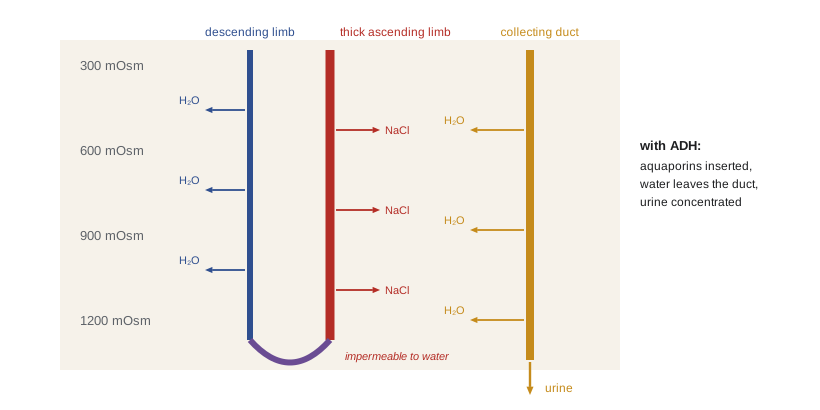
Mammals and birds are the only vertebrates that can produce urine more concentrated than their plasma. They do so with the loop of Henle, which works as a countercurrent multiplier. The thick ascending limb actively pumps sodium and chloride out of the tubule into the surrounding interstitial fluid, but its walls are impermeable to water, so the tubular fluid becomes more dilute and the interstitium more concentrated. The descending limb is permeable to water but not very permeable to salt, so water leaves the descending limb into the concentrated interstitium and the fluid inside becomes more concentrated as it descends. Because fluid flows in opposite directions in the two limbs, the small single effect of the pump at each level, about 200 mOsm, is multiplied along the length of the loop, building a gradient from about 300 mOsm in the cortex to 1,200 mOsm or more at the tip of the medulla in humans. Urea recycling between the collecting duct and the loop adds to the inner medullary gradient. The vasa recta, the capillaries that supply the medulla, are arranged as hairpin loops too, acting as countercurrent exchangers that remove reabsorbed water without washing out the gradient.
# Countercurrent multiplier: a simple stepwise model (after the classic textbook "single effect" demo)
# The loop is divided into N levels. Each step: (1) the ascending limb pumps salt so that
# the descending limb/interstitium at each level is 200 mOsm above the ascending limb;
# (2) fluid advances one level around the loop.
N, single_effect, steps = 8, 200.0, 60
desc = [300.0] * N        # descending limb (equilibrates with interstitium), top to bottom
asc = [300.0] * N         # ascending limb, bottom to top

for _ in range(steps):
    # flow: new 300 mOsm fluid enters the top of the descending limb,
    # fluid at the bottom turns the corner into the ascending limb
    bottom = desc[-1]
    desc = [300.0] + desc[:-1]
    asc = asc[1:] + [bottom]
    # single effect: at each level, move solute from ascending to descending side
    for i in range(N):
        total = desc[i] + asc[i]
        desc[i] = (total + single_effect) / 2
        asc[i] = (total - single_effect) / 2

print("level   descending/interstitium   ascending")
for i in range(N):
    print(f"  {i + 1}            {desc[i]:6.0f}              {asc[i]:6.0f}")
print(f"fluid leaving the ascending limb: {asc[0]:.0f} mOsm (dilute)")level descending/interstitium ascending 1 417 217 2 536 336 3 661 461 4 795 595 5 938 738 6 1094 894 7 1264 1064 8 1448 1248 fluid leaving the ascending limb: 217 mOsm (dilute)
Although the pump can create a difference of only 200 mOsm at any level, the gradient from the top to the bottom of the loop becomes much larger, and the fluid leaving the ascending limb is more dilute than plasma. Longer loops can build larger gradients, which is why the relative thickness of the renal medulla correlates with urine concentrating ability across mammals. The final concentration of the urine is set in the collecting duct. Antidiuretic hormone (vasopressin), released from the posterior pituitary when plasma osmolality rises or blood volume falls, causes water channels called aquaporin-2 to be inserted into the membranes of collecting duct cells. Water then leaves the duct into the concentrated medulla, and the urine becomes concentrated. Without the hormone, the duct is nearly impermeable to water and dilute urine is produced. Peter Agre's discovery of aquaporins earned a share of the 2003 Nobel Prize in Chemistry.
Hormonal control of salt and water
Several hormones act together. Aldosterone, from the adrenal cortex, increases sodium reabsorption and potassium secretion in the distal nephron and collecting duct. Its release is stimulated by angiotensin II, the end product of the renin–angiotensin system, which is activated when blood pressure or sodium falls. Angiotensin II also constricts blood vessels and stimulates thirst. Atrial natriuretic peptide, released when the heart's atria are stretched by high blood volume, has the opposite effects, promoting sodium and water excretion. In fish, cortisol and prolactin play leading roles in seawater and freshwater adaptation respectively, and birds and reptiles that drink sea water use salt glands near the eyes or tongue, controlled by the nervous system, to excrete concentrated salt solutions.
Desert animals
Desert rodents push water conservation to the limit. Kangaroo rats, studied in classic work by Knut and Bodil Schmidt-Nielsen in the Sonoran Desert of Arizona and nearby deserts, can live indefinitely on dry seeds without drinking. Merriam's kangaroo rat of the Mojave and Sonoran deserts is a favorite study animal, and Ord's kangaroo rat ranges across the Great Plains as far north as the prairies of Alberta and Saskatchewan. Kangaroo rats obtain most of their water from metabolic water, produced when food is oxidized, and lose very little: their very long loops of Henle produce urine of about 5,000 mOsm per kg or more, about four times as concentrated as human urine; their nasal passages cool exhaled air and recover water from it; they produce very dry feces; and they stay in humid burrows during the day. The Australian hopping mouse, Notomys, holds the record, with urine concentrations near 9,000 mOsm per kg.
Worked problem
Can a kangaroo rat live without drinking?
A 35 g kangaroo rat eats 5 g of dry seeds per day containing 10 percent water, 70 percent carbohydrate and 5 percent fat. Oxidizing 1 g of carbohydrate yields 0.56 g of metabolic water, and 1 g of fat yields 1.07 g. Its daily water losses are estimated at 1.9 g by evaporation, 0.6 g in urine and 0.2 g in feces. Is it in water balance?
Show solution
- Preformed water in food: 5 × 0.10 = 0.50 g.
- Metabolic water from carbohydrate: 5 × 0.70 × 0.56 = 1.96 g; from fat: 5 × 0.05 × 1.07 = 0.27 g; total about 2.23 g.
- Total water gain ≈ 0.50 + 2.23 = 2.73 g per day.
- Total water loss ≈ 1.9 + 0.6 + 0.2 = 2.7 g per day.
- Gain and loss are approximately equal, so the animal can balance its water budget without drinking, provided it stays in its humid burrow to keep evaporation low.
Answer: Yes, approximately. Metabolic water supplies over 80 percent of the intake, and the balance depends critically on keeping evaporative losses low; in dry air above ground, evaporation would rise and the budget would fail.
Common mistakes
MistakeAssuming marine fish have body fluids similar to sea water.
InsteadMarine teleosts keep their plasma at about a third of the osmolality of sea water and must drink and secrete salt.
MistakeConfusing osmolarity with tonicity.
InsteadOsmolarity counts all solutes; tonicity depends on which solutes cannot cross the membrane and thus affect cell volume.
MistakeThinking uric acid is excreted because it is the cheapest waste.
InsteadUric acid costs the most energy to make but saves water and suits development in shelled eggs.
MistakeSaying the loop of Henle makes urine concentrated by itself.
InsteadThe loop builds the medullary gradient; the final concentration depends on ADH-controlled water permeability of the collecting duct.
MistakeTreating filtration followed by reabsorption as wasteful.
InsteadIt lets the kidney excrete any substance not specifically reabsorbed, including novel toxins.
MistakeAssuming sharks are osmoconformers like sea stars.
InsteadSharks keep low plasma salt and retain urea and TMAO to raise osmolality slightly above sea water.
Summary and key terms
- Osmoregulation controls the water and salt content of body fluids; osmolarity counts solutes, tonicity describes effects on cells.
- Marine invertebrates conform; sharks retain urea balanced by TMAO; bony fish regulate at about a third of sea-water osmolality.
- Freshwater teleosts produce dilute urine and take up salt at gill ionocytes; marine teleosts drink and secrete salt at the gills.
- Smoltification prepares salmon for the sea under hormonal control; euryhaline fish switch gill transport patterns.
- Ammonia, urea and uric acid trade toxicity, water use and energy cost; the choice reflects habitat and development.
- Kidneys filter, reabsorb and secrete; the mammalian loop of Henle is a countercurrent multiplier, and ADH sets final urine concentration.
- Desert rodents combine long loops of Henle, metabolic water and behavior to live without drinking.
- osmolality
- The total concentration of osmotically active particles per kilogram of water.
- tonicity
- The effect of a solution on cell volume, depending on non-penetrating solutes.
- osmoconformer
- An animal whose body fluid osmolality matches its environment.
- counteracting solute
- An organic osmolyte, such as TMAO, that offsets the protein-destabilizing effect of another, such as urea.
- ionocyte
- A mitochondria-rich gill cell specialized for ion uptake or secretion.
- smoltification
- The physiological transformation that prepares young salmon for life in the sea.
- ornithine–urea cycle
- The metabolic pathway that converts ammonia to urea.
- Malpighian tubule
- An insect excretory tubule that forms primary urine by secretion.
- glomerulus
- A tuft of capillaries in the vertebrate kidney where blood is filtered.
- loop of Henle
- The hairpin segment of the mammalian and bird nephron that builds the medullary osmotic gradient.
- countercurrent multiplier
- A system in which a small transverse gradient is multiplied along a hairpin loop with opposite flows.
- antidiuretic hormone
- Vasopressin; it inserts aquaporins in the collecting duct to concentrate urine.
Practice problems
Work each problem on paper first, then reveal the answer to check.
What is the approximate osmotic pressure of a 0.3 osmolal solution at 25 °C?
Show answer
About 0.3 × 2.5 = 0.74 MPa.
Why can urea contribute to osmolality without much effect on cell volume?
Show answer
It crosses membranes readily, so it does not create a sustained osmotic gradient.
How do sharks avoid losing water to sea water?
Show answer
They retain urea and TMAO, raising plasma osmolality slightly above sea water.
List the main osmoregulatory problems and solutions of a marine teleost.
Show answer
Water loss and salt gain; it drinks sea water, absorbs water in the gut, and secretes NaCl at gill ionocytes and Mg²⁺/SO₄²⁻ in urine.
What changes occur during smoltification?
Show answer
Silvering, more seawater-type ionocytes, more gill sodium pumps, drinking, driven by cortisol, growth hormone and thyroid hormones.
Why do birds excrete uric acid?
Show answer
It saves water and can be stored safely as a precipitate in the shelled egg.
What happens to urine concentration when ADH is absent?
Show answer
The collecting duct stays impermeable to water and large volumes of dilute urine are produced.
Explain why the thick ascending limb must be impermeable to water.
Show answer
So that pumping salt out dilutes the tubular fluid and concentrates the interstitium instead of water simply following.
Why do kangaroo rats have exceptionally long loops of Henle?
Show answer
Longer loops multiply the single effect over a greater length, producing a steeper medullary gradient and more concentrated urine.
Name two sources of water for an animal that never drinks.
Show answer
Preformed water in food and metabolic water from oxidizing food.
Lesson quiz · 5 questions
Score 60% or more to complete this lesson.
Create a free account to save your progress, take quizzes and earn a certificate.